

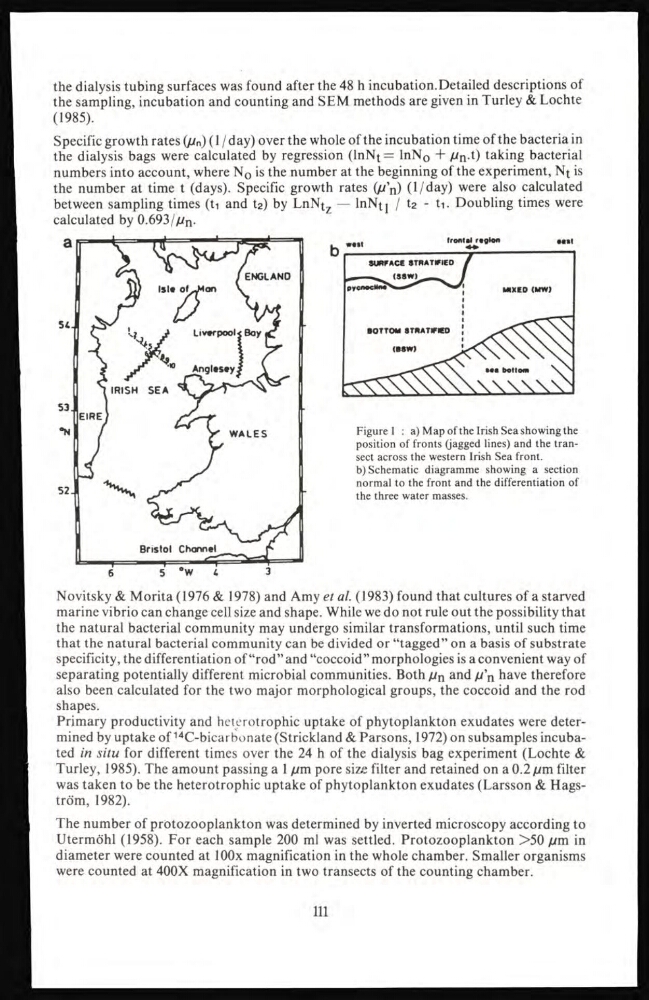
the dialysis tubing surfaces was found after the 48 h incubation.Detailed descriptions of
the sampling, incubation and counting and SEM methods are given in Turley & Lochte
(1985).
Specific growth rates (µ
n
) ( 1 / day) over the whole of the incubation time of the bacteria in
the dialysis bags were calculated by regression (1nNt= 1nN
O
+ µ
n
.t) taking bacterial
numbers into account, where N o is the number at the beginning of the experiment, N t is
the number at time t (days). Specific growth rates (µ' n ) (1/day) were also calculated
between sampling times (t
1
and t 2 ) by LnN tz — 1nN t1 / t
2
- t
1
. Doubling times were
calculated by 0.693/µ n .
Novitsky & Morita (1976 & 1978) and Amy et al. (1983) found that cultures of a starved
marine vibrio can change cell size and shape. While we do not rule out the possibility that
the natural bacterial community may undergo similar transformations, until such time
that the natural bacterial community can be divided or “tagged” on a basis of substrate
specificity, the differentiation of “rod” and “coccoid” morphologies is a convenient way of
separating potentially different microbial communities. Both µ n and µ’ n have therefore
also been calculated for the two major morphological groups, the coccoid and the rod
shapes.
Primary productivity and heterotrophic uptake of phytoplankton exudates were determined by uptake of
14 C-bicarbonate (Strickland & Parsons, 1972) on subsamples incubated in situ for different times over the 24 h of the dialysis bag experiment (Lochte &
Turley, 1985). The amount passing a 1 µm pore size filter and retained on a 0.2 µm filter
was taken to be the heterotrophic uptake of phytoplankton exudates (Larsson & Hagström, 1982).
The number of protozooplankton was determined by inverted microscopy according to
Utermöhl (1958). For each sample 200 ml was settled. Protozooplankton >50 µm in
diameter were counted at 100x magnification in the whole chamber. Smaller organisms
were counted at 400X magnification in two transects of the counting chamber.
Ill