

230
B. L. ASTAUROV
to this, more than 28 chromosome elements occur in the equatorial plates
of the primary spermatocyte division. Upon subsequent divisions there
invariably occurs an irregular distribution of the chromosomes passing
towards the poles, and this results in the formation of aneuploid spermatids and then spermatozoa, which is the cause of complete sterility of
males (Frolova's data in Astaurov, 1940; Kawaguchi, 1938b; Koshkina,
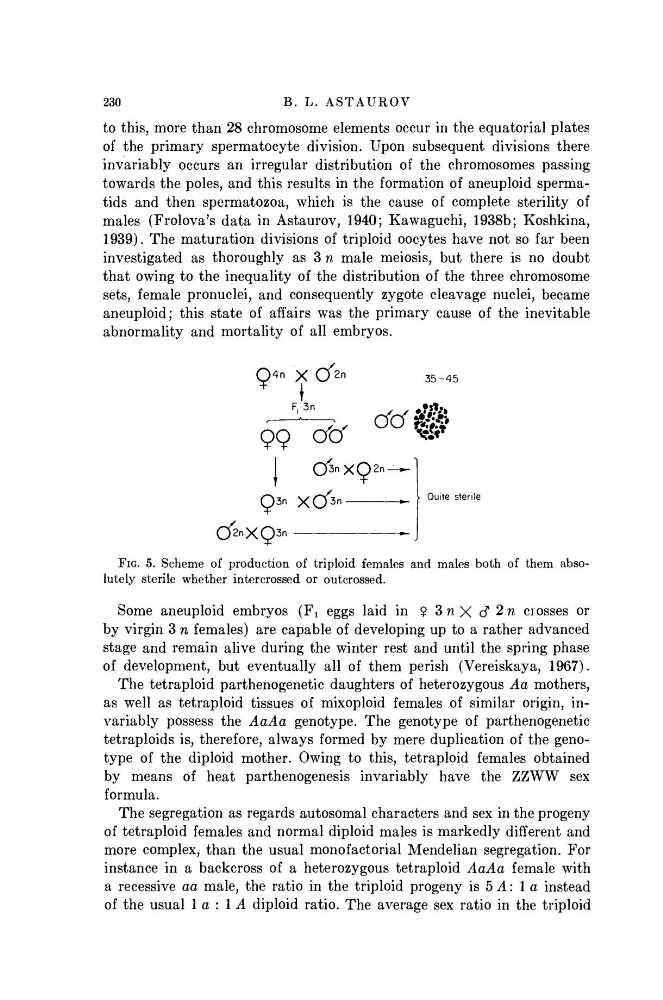
1939). The maturation divisions of triploid oocytes have not so far been
investigated as thoroughly as 3 n male meiosis, but there is no doubt
that owing to the inequality of the distribution of the three chromosome
sets, female pronuclei, and consequently zygote cleavage nuclei, became
aneuploid; this state of affairs was the primary cause of the inevitable
abnormality and mortality of all embryos.
Q
4
" X Cf
2n
35-45
F, 3n
çç cftf
93n XÖ2
Cfe*XQ
_ _ 3n ■
3n
Quite sterile
FIG. 5. Scheme of production of triploid females and males both of them absolutely sterile whether intercrossed or outcrossed.
Some aneuploid embryos (F 1 eggs laid in $ 3 n X c? 2 n crosses or
by virgin 3 n females) are capable of developing up to a rather advanced
stage and remain alive during the winter rest and until the spring phase
of development, but eventually all of them perish (Vereiskaya, 1967).
The tetraploid parthenogenetic daughters of heterozygous Aa mothers,
as well as tetraploid tissues of mixoploid females of similar origin, invariably possess the AaAa genotype. The genotype of parthenogenetic
tetraploids is, therefore, always formed by mere duplication of the genotype of the diploid mother. Owing to this, tetraploid females obtained
by means of heat parthenogenesis invariably have the ZZWW sex
formula.
The segregation as regards autosomal characters and sex in the progeny
of tetraploid females and normal diploid males is markedly different and
more complex, than the usual monofactorial Mendelian segregation. For
instance in a backcross of a heterozygous tetraploid AaAa female with
a recessive aa male, the ratio in the triploid progeny is 5 A : 1 a instead
of the usual 1 a : 1 A diploid ratio. The average sex ratio in the triploid