

THE ACRASINA
125
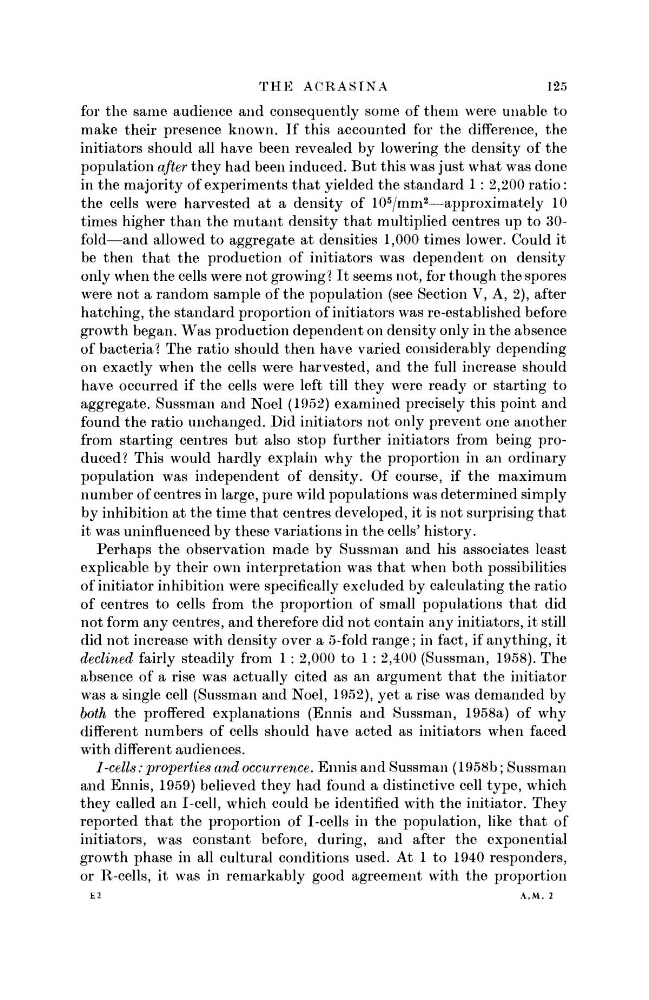
for the same audience and consequently some of them were unable to
make their presence known. If this accounted for the difference, the
initiators should all have been revealed by lowering the density of the
population after they had been induced. But this was just what was done
in the majority of experiments that yielded the standard 1 : 2,200 ratio:
the cells were harvested at a density of 10
5 /mm
2 —approximately 10
times higher than the mutant density that multiplied centres up to 30fold—and allowed to aggregate at densities 1,000 times lower. Could it
be then that the production of initiators was dependent on density
only when the cells were not growing? It seems not, for though the spores
were not a random sample of the population (see Section V, A, 2), after
hatching, the standard proportion of initiators was re-established before
growth began. Was production dependent on density only in the absence
of bacteria? The ratio should then have varied considerably depending
on exactly when the cells were harvested, and the full increase should
have occurred if the cells were left till they were ready or starting to
aggregate. Sussman and Noel (1952) examined precisely this point and
found the ratio unchanged. Did initiators not only prevent one another
from starting centres but also stop further initiators from being produced? This would hardly explain why the proportion in an ordinary
population was independent of density. Of course, if the maximum
number of centres in large, pure wild populations was determined simply
by inhibition at the time that centres developed, it is not surprising that
it was uninfluenced by these variations in the cells' history.
Perhaps the observation made by Sussman and his associates least
explicable by their own interpretation was that when both possibilities
of initiator inhibition were specifically excluded by calculating the ratio
of centres to cells from the proportion of small populations that did
not form any centres, and therefore did not contain any initiators, it still
did not increase with density over a 5-fold range; in fact, if anything, it
declined fairly steadily from 1 : 2,000 to 1 : 2,400 (Sussman, 1958). The
absence of a rise was actually cited as an argument that the initiator
was a single cell (Sussman and Noel, 1952), yet a rise was demanded by
both the proffered explanations (Ennis and Sussman, 1958a) of why
different numbers of cells should have acted as initiators when faced
with different audiences.
I-cells: properties and occurrence. Ennis and Sussman (1958b; Sussman
and Ennis, 1959) believed they had found a distinctive cell type, which
they called an I-cell, which could be identified with the initiator. They
reported that the proportion of I-cells in the population, like that of
initiators, was constant before, during, and after the exponential
growth phase in all cultural conditions used. At 1 to 1940 responders,
or R-cells, it was in remarkably good agreement with the proportion
E2
A , M . 2